MIM complex
A protein complex located in the mitochondrial outer membrane that functions as an insertase, mediating the insertion of alpha-helical proteins from the cytosol into the outer membrane. Client proteins are usually single- and multi-span proteins that include components of the TOM complex. [GO:0140595]
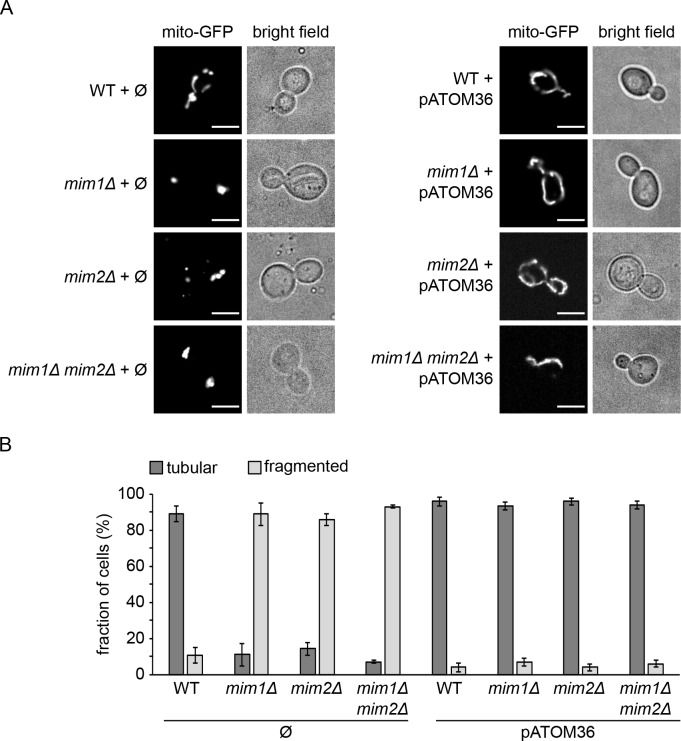
NCBITaxon:4932) · Daniela G Vitali, Sandro Käser, Antonia Kolb, Kai S Dimmer, Andre Schneider, Doron Rapaport; CC BY, via PubMed Central · CC_BY_4_0 · source: PMC PMC6010339.1 fig5 · DOI:10.7554/eLife.34488Synonyms: mitochondrial outer import machinery
Part of: mitochondrial outer membrane (GO:0005741)
Components
| Component | Type | Part of / acts on | Grounding | Genes | Stoichiometry | Essential | Role |
|---|---|---|---|---|---|---|---|
| Outer membrane protein, MIM1/TOM13, mitochondrial | Protein | part of | InterPro:IPR013262 | MIM1, TOM13 | Mim1 subunit of the mitochondrial outer-membrane alpha-helical protein import complex.
| ||
| Mim2 | Protein | part of | InterPro:IPR037652 | MIM2 | Partner subunit of Mim1 in the mitochondrial outer-membrane import complex.
|
Taxonomic distribution
NCBITaxon:4932Saccharomyces cerevisiae — COMMON: Experimentally characterized in budding-yeast YPH499 derivatives; no universal fungal or eukaryotic distribution is asserted. [DOI:10.1016/j.celrep.2020.107567]
Canonical examples
NCBITaxon:4932Saccharomyces cerevisiae — YPH499-derived strains provide isolated-mitochondrial import, affinity-purification and native-gel evidence. The separate 2018 deletion/rescue microscopy uses W303 derivatives. Heterologous expression in Trypanosoma brucei is not evidence for a native trypanosome MIM complex. [DOI:10.1016/j.celrep.2020.107567]
Functions
- alpha helical protein insertion into mitochondrial outer membrane
GO:7770059— Promotes biogenesis of selected signal-anchored, tail-anchored and multispanning alpha-helical mitochondrial outer-membrane proteins; dependence varies with substrate and assay.DOI:10.1016/j.celrep.2020.107567Radiolabeled precursor import, mim1-23 controls and precursor co-purification support an import role. Fis1 and Gem1 import are impaired under these isolated-mitochondrial assay conditions; these results do not prove an exclusive route.DOI:10.1016/j.isci.2019.100779Msp1 import is strongly MIM dependent, Gem1 is only moderately dependent, and Fis1 and Mcr1 mitochondrial levels are largely MIM independent. This preserves the contrast with the later import assays.DOI:10.7554/eLife.34488Loss of Mim1/Mim2 impairs Tom20 and Ugo1 import. Heterologous pATOM36 rescues Tom20 much more effectively than Ugo1, so functional interchangeability is substrate limited.
Mechanism graphs
MIM-dependent import and distinct TOM/SAM-associated populations (FUNCTION)
MIM promotes selected precursor-import and assembly reactions and associates separately with TOM and SAM.
| Subject | Predicate | Object | Evidence |
|---|---|---|---|
| MIM complex | associates with | mitochondrial outer membrane translocase complex |
|
| MIM complex | associates with | SAM complex |
|
| MIM complex | promotes | Import of tested signal-anchored precursors |
|
| MIM complex | promotes | Import of tested tail-anchored precursors |
|
| MIM complex | promotes formation of | SAM-associated Tom6 assembly intermediate |
|
Discussions
- INTERPRETATION (RESOLVED): Distinguish MIM constituents from interacting import systems, substrates and functional substitutes. TOM and SAM association, precursor binding and heterologous rescue do not establish additional constitutive MIM components.
- CONTROVERSY (OPEN): Resolve the assay-dependent differences in Fis1 and Mcr1 dependence on MIM. The iScience study finds largely preserved mitochondrial levels of Fis1 and Mcr1 and only minor Fis1 mistargeting, whereas the later Cell Reports import assays detect MIM-dependent effects. Steady-state abundance, targeting fidelity and import kinetics are different readouts; these sources do not establish which experimental differences explain the contrast.
- CURATION_TODO (OPEN): Resolve native MIM stoichiometry and the proposed exchange between free, TOM-associated and SAM-associated populations. Native-gel migration and complementation do not resolve an intact atomic structure or fixed copy number. Competition and altered association support a dynamic-exchange model without directly observing exchange. The hosted microscopy shows organelle morphology, not molecular MIM localization or structure.
Evidence
DOI:10.1016/j.celrep.2020.107567Doan et al. (2020), The Mitochondrial Import Complex MIM Functions as Main Translocase for alpha-Helical Outer Membrane Proteins. Main text, Figures 1-4 and experimental methods inspected in the institutional publisher PDF. CC BY-NC-ND: figures not hosted.DOI:10.7554/eLife.34488Independent evolution of functionally exchangeable mitochondrial outer membrane import complexes. Relevant yeast and heterologous Results, Discussion, strain/microscopy methods and Figure 5 inspected in checksum-verified PMC6010339 version 1.DOI:10.1016/j.isci.2019.100779The Biogenesis of Mitochondrial Outer Membrane Proteins Show Variable Dependence on Import Factors. Signal-anchored and tail-anchored Results, Discussion and limitations inspected in checksum-verified PMC6965732 version 1.GO:0098799Broader is-a parent: outer mitochondrial membrane protein complex.GO:0005741Containing mitochondrial outer membrane, not an is-a parent.
Curation history
2026-10-04T23:11:03Zcodex · CREATED_RECORD — Scaffolded by scripts/new_record.py2026-10-04T23:13:24Zcodex · EXPANDED_RECORD — Added verified Mim1/Mim2 families, yeast-bounded examples, exact GO insertion function, five source-cited functional edges and explicit substrate-dependence, partner-boundary and architecture limits.2026-10-04T23:14:29Zpmc_oa · ADD_IMAGE — Added PMC6010339.1 fig5; version, CC licence, JATS figure identity and media md5 verified through the PMC OA S3 dataset.